Research Insight
Effects of Different Pinching Treatments on Branch Formation and Flower Yield of Chrysanthemum morifolium 

 Author Correspondence author
Genomics and Applied Biology, 2026, Vol. 17, No. 5 doi: 10.5376/gab.2026.17.0023
Received: 08 Aug., 2026 Accepted: 12 Sep., 2026 Published: 26 Sep., 2026
Jiang C.B., 2026, Effects of different pinching treatments on branch formation and flower yield of Chrysanthemum morifolium, Genomics and Applied Biology, 17(5): 299-311 (doi: 10.5376/gab.2026.17.0023)
Topping is an important cultivation practice for regulating plant architecture, branching development, and flower production in chrysanthemum. However, the effects of different topping methods on branch formation and flower yield in Hangbaiju (Chrysanthemum morifolium Ramat.) remain insufficiently understood. This review systematically examines the effects of topping timing, intensity, and frequency on vegetative growth, axillary bud development, canopy structure, photosynthetic performance, flower bud differentiation, and yield formation in Hangbaiju. Topping can alleviate apical dominance and stimulate axillary bud outgrowth, thereby increasing the number and complexity of primary and secondary branches. Appropriate topping may improve canopy architecture, enhance light interception and photosynthetic productivity, and promote assimilate accumulation and allocation toward reproductive organs. In contrast, excessive or improperly timed topping may delay plant development, reduce photosynthetic source capacity, and adversely affect flower bud formation and final yield. A representative case study framework is proposed to evaluate different topping treatments based on plant morphology, branching characteristics, flowering traits, and yield components. Integrating physiological responses with yield-related indicators can facilitate the identification of optimal topping strategies. Overall, moderate and appropriately timed topping is expected to provide an effective approach for coordinating branching, canopy development, and flower production, offering a theoretical basis for precision cultivation and standardized production of Hangbaiju.
1 Introduction
Hangbaiju, a cultivated form of Chrysanthemum morifolium, has production value that extends beyond ornamental use because it is widely cultivated and economically important in China, while even its leaf residues contain recoverable polyphenols with antioxidant potential and value-added processing prospects (Yuan et al., 2025). More broadly, chrysanthemum has become an important commercial floricultural crop because of its uses as a pot plant, loose flower, cut flower, and landscape species, and this multifunctionality has supported rapid expansion of its production and trade in diverse regions. The commercial importance of chrysanthemum also means that cultivation is judged not only by whether plants flower, but by whether they produce the branching pattern, flower number, flower size, and harvest timing required by different markets. In practical production, this creates a need for cultivation strategies that can coordinate vegetative architecture with reproductive output, especially in forms grown for numerous harvestable capitula rather than a few large blooms (Kumar et al., 2024). For Hangbaiju, whose harvested flower heads determine much of its direct economic return, management practices that increase productive shoots and stabilize inflorescence yield are therefore closely tied to industrial development and grower profitability.
Among such practices, topping or pinching is especially important because it directly alters apical dominance and redistributes growth toward lateral buds. Chrysanthemum studies consistently show that unpinched plants tend to be taller and earlier flowering, whereas pinched plants usually become shorter, wider, and more branched (Kathad et al., 2024). The basic mechanism has been described similarly across experiments: removal of the terminal growing point suppresses apical dominance, promotes axillary bud outgrowth, and redirects assimilates toward side shoots, thereby increasing branch number and canopy spread. This architectural shift is important because flower number in chrysanthemum is strongly linked to the number of productive lateral shoots, so treatments that enhance branching often improve flower production per plant. Quantitative studies support that pattern: pinching at 30 days after transplanting increased branches and flower yield in annual chrysanthemum, while double or repeated pinching often produced even more branches and flowers than no pinching. At the same time, the response is not one-dimensional. No pinching can advance bud initiation and flowering and often gives larger individual flowers, whereas more intensive pinching tends to delay flowering and reduce single-flower size even as total flower number rises (Mohanty et al., 2025). Some studies likewise show that double pinching maximizes flower count but not necessarily flower yield by weight or economic return, because single pinching at the right stage can outperform double pinching for total harvested mass and benefit-cost ratio). This means the agronomic value of topping depends not only on whether pinching is applied, but on how many times it is done and when it is imposed.
That variability is exactly why research on different topping methods remains necessary for Hangbaiju. Existing chrysanthemum evidence shows that the optimal pinching regime differs with genotype, production target, and associated cultivation conditions. In Chrysanthemum morifolium cv. Ratlam Selection, pinching at 30 days after transplanting promoted branch number and plant spread, indicating that early topping can strongly improve branch formation in the same species targeted here. In other chrysanthemum types, however, double pinching produced the highest numbers of flowers or branches, while single pinching sometimes gave the best balance among yield, flower quality, and plant form. Studies that combined pinching with growth regulators or nitrogen further indicate that topping effects interact with crop management background, affecting not only branching but also leaf area, stem thickness, flowering span, and total yield. This broader evidence suggests that a topping treatment cannot be assumed optimal across all production systems, and recommendations developed for annual chrysanthemum, spray chrysanthemum, or pot types may not transfer directly to Hangbaiju grown for capitulum harvest. A focused study on different topping methods in Hangbaiju is therefore significant for both theory and practice: theoretically, it helps clarify how manipulation of apical control shapes branch formation and yield allocation in C. morifolium; practically, it can identify a topping regime that improves flower-head production while balancing flowering time and plant architecture for commercial cultivation. On that basis, the present study examines the effects of different pinching treatments on branch formation and flower yield of Chrysanthemum morifolium to provide a more targeted foundation for efficient Hangbaiju production.
2 Biological Basis of Growth and Branch Formation in Hangbaiju
2.1 Characteristics of vegetative and reproductive growth in Hangbaiju
Hangbaiju is a perennial short-day chrysanthemum in which vegetative growth and reproductive transition are tightly connected to production performance. In chrysanthemum, substantial variation exists in plant height, spread, branching, and flowering behavior among genotypes, indicating that branch architecture is a biologically variable trait rather than a fixed cultivar feature (Bala and Kaur, 2026). In Hangbaiju specifically, flowers are borne at the tops of branches, so shoot architecture directly determines the capacity for reproductive output and final harvestable flower number.
The transition from vegetative to reproductive growth also changes the pattern of meristem activity along the shoot. In one chrysanthemum genotype that underwent floral transition, the apex shifted from vegetative growth at the early stage to floral transition and then stopped initiating new axillary buds, showing that reproductive development restructures further branch initiation potential. Photoperiod studies support the same trade-off, because conditions favoring stronger vegetative growth increased branch and leaf formation, whereas greater flower induction tended to coincide with reduced branch or leaf production as resources and developmental priority shifted toward reproduction (Yang et al., 2024).
2.2 Apical dominance and axillary bud development
The biological basis of branch formation in chrysanthemum begins with apical dominance, whereby the active shoot tip suppresses outgrowth of axillary buds below it. During vegetative growth, chrysanthemum plants show short inhibited buds near the apex, and this pattern is a direct expression of apical control over lateral development. More generally, axillary branch development proceeds through bud formation, bud release or dormancy, and bud elongation, so the visible branch number observed after pinching reflects regulation at multiple developmental stages rather than only a single bud-break event (Figure 1).
|
Figure 1 Biological basis of apical dominance release and axillary branch formation in chrysanthemum. The schematic illustrates the transition from shoot-apex-mediated inhibition to axillary bud release and subsequent lateral shoot elongation following pinching or decapitation, with coordinated regulation by auxin, cytokinins, sugars, strigolactones, gibberellins, and chrysanthemum branching-related genes |

This control system is mediated by interacting hormonal and carbohydrate signals. In chrysanthemum, release from apical dominance after floral transition coincided with decreased auxin and increased cytokinin levels in subapical buds, together with altered expression of branching regulators such as CmBRC1, CmDRM1, and CmMAX1. Broader apical-dominance research shows that auxin does not act alone, because sugars can trigger rapid cytokinin increases after decapitation, strigolactones mainly constrain later sustained growth rather than the earliest release step, and branching emerges from a network involving auxin, cytokinin, strigolactones, sugars, and gibberellins (Cao et al., 2023).
2.3 Relationship between branch number and inflorescence formation
The number of branches is closely tied to inflorescence formation because chrysanthemum flowers are produced terminally on shoots, making each successful lateral branch a potential flowering unit. In Hangbaiju, the importance of this link is explicit: the number of shoot branches is considered crucial for achieving high flower yield, which is why manual decapitation has traditionally been used to stimulate branching despite its labor cost. Across chrysanthemum production studies, treatments that increase branch number commonly increase flower number per plant as well, confirming that branch proliferation usually expands the population of reproductive sites (Jena et al., 2021).
The relationship is positive but not unlimited, because branch promotion also changes flowering time and the allocation of assimilates among floral units. Pinching studies show that double or repeated pinching increases primary branching and raises flower number and flower yield, but it often delays flowering and can reduce individual flower size compared with unpinched plants (Das and Patra, 2025). Nutrient and light-environment studies add that inflorescence productivity depends on how well branch formation is supported by whole-plant growth conditions, since balanced fertilization can enhance branching and flowering traits, and side lighting can markedly increase branch number while simultaneously promoting flowering and morphophysiological performance. Overall, the biological basis of branch formation in Hangbaiju is a coordinated system in which vegetative vigor, release from apical dominance, and conversion of lateral shoots into flower-bearing branches jointly determine yield. This is why different pinching treatments can produce large differences in flower production: they intervene directly in the developmental network that links shoot architecture to reproductive output.
3 Cultivation and Regulatory Mechanisms of Different Topping Methods
3.1 Effects of single topping on plant architecture
Single topping primarily alters plant architecture by removing the terminal bud, weakening apical dominance, and redirecting growth toward lateral shoots. In potted chrysanthemum, one terminal-bud pinching reduced final plant height relative to the unpinched control while increasing leaf number, branch number, and flowers per plant, showing that a single intervention can already shift plants from vertical growth to a more compact and productive canopy. A similar architectural response was recorded in Chrysanthemum morifolium cv. Ratlam Selection, where pinching at 30 days after transplanting produced the maximum number of branches and the greatest plant spread among the tested pinching times.
Single topping also affects reproductive rhythm by trading earlier flowering for improved lateral development. In annual chrysanthemum, no pinching gave the largest flowers and earliest bud appearance, whereas single pinching improved canopy spread and still maintained favorable flower characters compared with more intensive pinching. Another factorial study found that single pinching at 15 days after transplanting gave the highest flower weight and earliest 50% flowering, while single pinching at 30 days ranked next and produced broader plant spread, indicating that one well-timed topping can balance architecture and yield without the stronger flowering delay associated with repeated pinching (Mohanty et al., 2025).
3.2 Effects of multiple topping and hierarchical pruning
Multiple topping strengthens the branching response by repeatedly interrupting apical dominance, thereby increasing the number of active lateral growing points and expanding canopy spread. In Chrysanthemum indicum, three pinching events produced the highest branch number, leaf number, plant spread, and flower number, while unpinched plants remained the tallest and least branched (Ehsanullah et al., 2021). In annual chrysanthemum, double pinching likewise produced the shortest plants but the greatest numbers of leaves, primary branches, and flowers per plant, supporting the general rule that repeated topping shifts assimilate use away from main-stem elongation and toward branch proliferation.
Hierarchical pruning effects depend not only on pinching frequency but also on which node positions are retained after each cut. In garland chrysanthemum, new-shoot emergence after the first pinching was higher than after the second, and lateral-shoot development varied systematically with node position (Matsunaga and Sasaki, 2026). Shoots arising from the first and second nodes of the main stem showed stronger subsequent regeneration, whereas regrowth from lower nodes on upper first-order laterals was weaker, indicating that hierarchical pruning should retain node positions with higher regenerative capacity rather than treating all lateral shoots as equivalent.
3.3 Interactive effects of topping intensity and timing
The effect of topping intensity depends strongly on timing, because earlier and later pinching modify different developmental phases of the crop. In garland chrysanthemum, pinching in the nursery at 20 days after sowing produced the highest branch number, plant spread, and stem girth, whereas non-pinched plants stayed consistently taller, showing that early topping can be more effective for branch induction than delayed intervention. In C. morifolium cv. Ratlam Selection, pinching at 30 days after transplanting outperformed pinching at 45 days for branch number and plant spread, while no pinching still led to earlier bud initiation and 50% flower opening, which highlights the trade-off between structural improvement and earliness.
Increasing topping intensity can further raise flower number, but delayed or repeated pinching often postpones flowering and may reduce individual-flower traits. In annual chrysanthemum, double pinching at 15 and 30 days gave the highest flower number, but it also significantly delayed flowering and reduced individual flower size. Tea-applied chrysanthemum showed a related pattern at the production scale: two-time pinching produced the highest crown width, flower number, fresh mass, yield per plant, and yield per unit area, while postponing pinching reduced plant height, and a separate factorial study found that the statistical interaction between planting time and pinching was non-significant for measured flowering and yield traits, suggesting that pinching timing matters greatly but does not always interact strongly with calendar planting date (Thumar et al., 2020). Overall, different topping methods regulate Hangbaiju through a common developmental mechanism: removal of terminal dominance promotes lateral shoot growth, but the agronomic outcome depends on how many times, how early, and at which hierarchical positions the plant is pinched. For practical flower production, single topping tends to provide a balanced canopy response, whereas repeated or hierarchically optimized topping is more suitable when maximizing branch number and total flower yield is the primary goal.
4 Effects of Topping Treatments on Branch Formation and Canopy Structure of Hangbaiju
4.1 Changes in plant height, stem diameter, and internode characteristics
Topping consistently suppresses vertical elongation in chrysanthemum by removing the active apex and weakening apical dominance, so unpinched plants generally remain the tallest while topped plants become shorter and more compact. In annual chrysanthemum, no pinching produced the greatest plant height, whereas pinching at 30 or 40 days after transplanting significantly reduced height, showing that even a single topping event can redirect growth away from the main axis (Nagdeve et al., 2021). More intensive topping strengthens that effect, as thrice-pinched plants were much shorter than unpinched controls in field-grown chrysanthemum. A similar pattern appears in treatment combinations with growth regulators, where double pinching at 25 and 40 days gave the shortest plants, again indicating that repeated apex removal limits internode extension.
Stem thickening and shortening of the canopy framework often accompany reduced plant height after topping. Pinching at 40 days increased stem girth compared with no pinching in annual chrysanthemum, suggesting that reduced longitudinal growth is associated with stronger radial development. A newer study likewise found that pinching increased stem diameter while no pinching maintained the greatest height, reinforcing the trade-off between elongation and structural robustness (Mangulal et al., 2025). Internode behavior follows the same trend, because the longest internodal distance was recorded in unpinched plants, while stronger pinching shifted plants toward shorter, denser shoot architecture. Nitrogen-interaction results support this interpretation: maximum stem diameter, branch number, plant spread, and leaf area occurred under pinching with adequate nitrogen rather than under the tallest no-pinching treatment.
4.2 Formation of primary, secondary, and higher-order branches
The most direct architectural consequence of topping is the release of axillary buds, which increases the number of primary branches and creates the structural basis for secondary and tertiary branching. In Chrysanthemum morifolium cv. Ratlam Selection, pinching at 30 days after transplanting produced the highest branch number throughout growth, consistent with the view that early apex removal stimulates lateral bud outgrowth. In another chrysanthemum study, pinching increased primary and secondary branch numbers together with stem diameter and plant spread, showing that lateral activation is not confined to one branch order. Hormone evidence supports the same mechanism: cytokinin treatment increased chrysanthemum branch number and lateral bud diameter, whereas auxin and strigolactone treatments inhibited branching (Wang et al., 2024).
As topping intensity rises, branch hierarchy becomes progressively more complex, but the strongest increase in branch order does not always coincide with the best overall flower yield. Double pinching maximized primary branches and flower number in annual chrysanthemum, indicating that two sequential releases from apical control can amplify reproductive shoot formation. In spray-type chrysanthemum, pinching three times at 30, 40, and 50 days produced the highest primary, secondary, and tertiary branch numbers, demonstrating a clear cumulative effect of repeated pruning on branch hierarchy. Genetic and architectural analyses further show that upper primary branch number and total lateral bud production are highly variable chrysanthemum traits and are sensitive to environment, which helps explain why topping responses differ among cultivars and production systems (Sun et al., 2022). Even so, branch proliferation has practical limits, because larger individual flowers are often retained in unpinched controls while more heavily pinched plants distribute assimilates across a greater number of flowering shoots.
4.3 Canopy structure and light energy utilization
Once topping increases lateral branching, its importance extends beyond branch number to the three-dimensional structure of the canopy. In flower crops, canopy architecture regulates microclimate, light interception, and resource-use efficiency, and traits such as plant height, branching pattern, and foliage distribution determine how light is distributed within the canopy (Nateshkumar et al., 2025). This is directly relevant to Hangbaiju because topping changes exactly those structural traits, especially canopy width and branch arrangement. Studies in chrysanthemum repeatedly show that pinching increases plant spread, with early pinching often producing the broadest canopy and repeated pinching producing the most expanded crown.
Broader canopy-physics studies clarify why these structural changes matter for light-energy utilization. Light interception and biomass production depend not only on total leaf area but on how radiation penetrates the canopy, with smaller or more open canopies often showing better penetration per unit leaf area, while excessive mutual shading reduces efficiency. Branch angle, internode spacing, and pruning pattern also alter light capture, and simulated canopies show that pruning and reshaping can improve PAR distribution and photosynthetic performance by reducing self-shading (Ran, 2025). Crop-level evidence reaches the same conclusion: optimizing canopy structure improves photosynthesis and yield by improving light-interception distribution within the stand rather than merely increasing vegetative mass. Overall, Hangbaiju topping treatments influence yield formation through a linked sequence of effects: reduced main-stem elongation, enhanced multi-order branching, and reorganized canopy light capture. The most favorable treatment is therefore unlikely to be the one that produces either the tallest plants or the greatest branch number alone, but the one that builds a canopy with efficient branch distribution and effective internal light use.
5 Effects of Topping Methods on Physiological Characteristics and Flower Bud Formation in Hangbaiju
5.1 Leaf photosynthetic characteristics and assimilate accumulation
Different topping methods influence leaf physiological status mainly by changing source–sink balance and canopy development. Pinching generally increases leaf number, and repeated pinching often produces the largest leaf display, indicating stronger assimilatory surface development than in unpinched plants (Ehsanullah et al., 2021). In combination treatments, double pinching also increased leaf area, leaf area index, and leaf area duration, showing that topping can extend the functional photosynthetic surface available for assimilate production.
These structural changes are accompanied by physiological adjustments associated with assimilate accumulation. Single pinching produced the highest leaf area in one annual chrysanthemum study, whereas double pinching maximized branch proliferation, suggesting that moderate topping can favor leaf-level assimilatory capacity while stronger topping favors redistribution into new sinks. Leaf chlorophyll intensity also increased under repeated pinching, which supports the view that topping can enhance the photosynthetic competence of remaining foliage even while delaying reproductive advance.
5.2 Carbon and nitrogen metabolism and dry matter allocation
The effects of topping on carbon and nitrogen metabolism are best understood through changes in assimilate redistribution after the shoot apex is removed. Pinching redirects carbohydrates toward axillary buds and developing lateral shoots, which explains the common increase in branching and canopy expansion after treatment. A related flowering-yield study similarly noted that in pinched plants, energy was shared among developing side branches rather than being concentrated mainly in the main stem, indicating a basic shift in assimilate allocation pattern.
Chrysanthemum dry-matter studies show why this redistribution matters for flower production. During normal growth, dry-matter accumulation continues through inflorescence development, and the developing inflorescence becomes a strong assimilate sink, while nitrogen accumulation peaks earlier and later demand is increasingly met by remobilization from vegetative tissues. Nitrogen-management research further shows that better photosynthetic function and higher light availability can improve nitrogen-use efficiency, water-use efficiency, and allocation of biomass toward flowers, while predictive modeling confirms that aboveground dry matter and nitrogen accumulation are tightly linked across the chrysanthemum growth period (Liu et al., 2025).
5.3 Flower bud differentiation and flowering progression
Topping affects flower bud differentiation primarily by postponing the reproductive transition while increasing the number of potential flowering sites. Across chrysanthemum studies, no pinching consistently resulted in the earliest flower bud appearance, whereas repeated pinching delayed bud initiation because plants re-entered or prolonged vegetative development after apex removal. This delay can become substantial under stronger treatments, with twice or thrice pinched plants showing longer periods to inflorescence bud formation and later 50% flowering than unpinched controls.
Even though bud initiation is delayed, the later flowering phase often becomes more productive and more extended. Double pinching increased flower number and total yield in annual chrysanthemum, indicating that delayed bud differentiation is compensated by the formation of more reproductive shoots. Other studies show the same developmental trade-off: double pinching delayed flowering progression but increased branch number, flowers per stem, flowering span, and total flower yield, whereas single pinching more often balanced flowering quality and display uniformity (Kaur and Singh, 2024). Overall, different topping methods influence Hangbaiju not only through visible architectural change but through coordinated shifts in leaf function, assimilate partitioning, and timing of reproductive development. In practice, lighter topping tends to preserve earlier flowering and stronger individual-organ performance, whereas repeated topping tends to favor cumulative branch formation and total flower production.
6 Case Study: Effects of Different Topping Methods on Branch Formation and Flower Yield of Hangbaiju
6.1 Case study design and experimental treatments
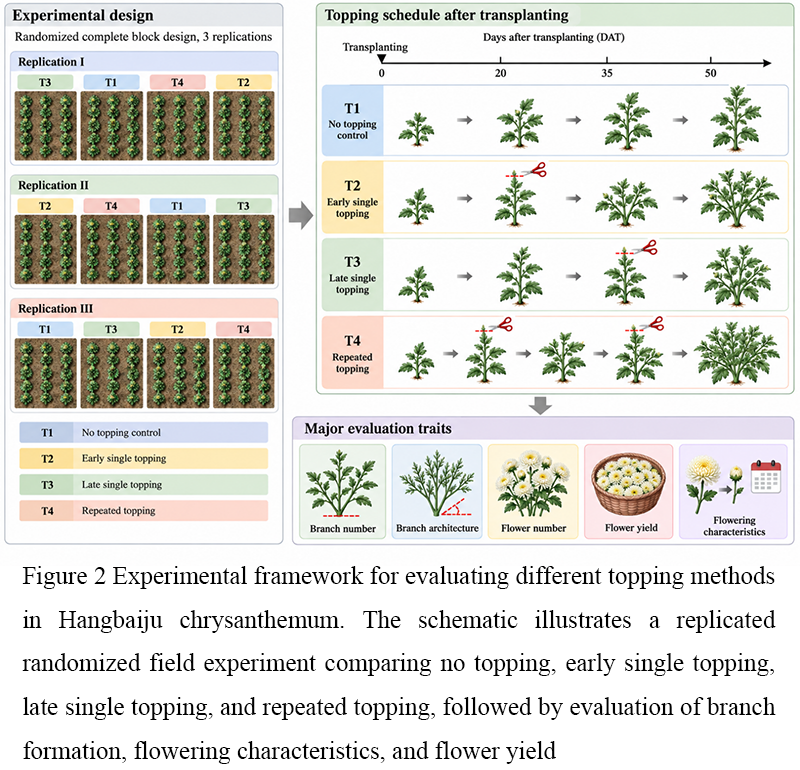
A case study on different topping methods in Hangbaiju should be framed as a comparative experiment in which branch formation and flower yield are evaluated under clearly defined pinching schedules. Existing chrysanthemum studies commonly use randomized designs with replicated treatment combinations, such as factorial randomized block designs with three replications and treatments contrasting no pinching with one or more topping times after transplanting. This structure is appropriate for Hangbaiju because flower production depends strongly on branch number, and Hangbaiju cultivation has traditionally relied on repeated manual decapitation to increase shoot branching (Zhang et al., 2023).
The treatment system should include at least a control without topping, a single early topping treatment, a single later topping treatment, and one repeated topping treatment, because these contrasts recur across the chrysanthemum literature and capture the main agronomic decision points. For example, studies have compared no pinching with pinching at 30 or 40 days after transplanting, while others have extended the range to twice or thrice pinching treatments to test increasing intensity (Ehsanullah et al., 2021). Similar design logic has also been used in tea-applied chrysanthemum, where different pinching schemes were evaluated together with planting-date effects in a split-split plot field experiment, showing that topping pattern itself can be treated as a main analytical factor (Figure 2).
|
Figure 2 Experimental framework for evaluating different topping methods in Hangbaiju chrysanthemum. The schematic illustrates a replicated randomized field experiment comparing no topping, early single topping, late single topping, and repeated topping, followed by evaluation of branch formation, flowering characteristics, and flower yield |
6.2 Responses of branch formation and flower yield
The expected response pattern in Hangbaiju is that topping reduces apical dominance, increases branch production, and then raises the number of flower-bearing shoots, although the strongest treatment is not always the one that produces the highest marketable yield. In Chrysanthemum morifolium cv. Ratlam Selection, pinching at 30 days after transplanting increased branch number and plant spread relative to no pinching, showing the value of timely apex removal for canopy expansion. In tea-applied chrysanthemum, two-time pinching increased crown width, flower number, fresh mass, yield per plant, and yield per unit area over no pinching, while also markedly reducing plant height.
More intensive topping can further increase branch hierarchy and flower number, but it often delays flowering and may not optimize all yield components simultaneously. In annual chrysanthemum, double pinching produced the maximum primary branches and flower yield and was recommended for commercial yield maximization. By contrast, in spray chrysanthemum cv. Shyamal, thrice pinching produced the best vegetative branching traits, but the highest flower number and yield by weight were achieved with pinching twice at 30 and 40 days after transplanting (Das and Patra, 2025).
6.3 Correlations among key traits and selection of the optimal topping method
Trait relationships in a Hangbaiju case study should be interpreted around one central biological link: more effective branch formation usually increases the number of terminal flowering sites, but this advantage must be balanced against flowering delay and changes in single-flower quality. In Hangbaiju itself, shoot branch number is described as crucial for achieving high flower yield because flowers are borne at the tops of branches. Supporting evidence from annual chrysanthemum shows that pinching-induced increases in flower number are associated with vegetative traits such as increased branch number, indicating a positive correlation between branching capacity and reproductive output.
Selection of the optimal topping method should therefore prioritize the treatment that gives the best integrated balance among branch number, canopy spread, flower number, and harvestable yield rather than the tallest plants or the earliest flowering alone. Some systems favor relatively early single pinching, as shown by the Punjab study where pinching at 40 days combined with GA3 produced the highest branch number, leaf number, flower number, and yield per hectare among the tested combinations. Other systems favor moderate repeated topping, and even non-chrysanthemum evidence points in the same direction, with marigold showing maximum flower number and branching under later pinching rather than the unpinched control (Chandio et al., 2023). For Hangbaiju, the most reasonable conclusion is that the optimal topping method is the one that maximizes productive branching without imposing excessive delay or over-fragmenting assimilates among too many shoots. A case study built on these comparisons would therefore be well positioned to identify whether single early topping or two-time topping gives the best balance for branch formation and flower yield in Chrysanthemum morifolium.
7 Integrated Mechanisms Underlying the Effects of Different Topping Methods on Flower Yield
7.1 Release of apical dominance and branching compensation
Different topping methods first act by removing the active shoot apex, thereby weakening apical dominance and releasing suppressed axillary buds. In chrysanthemum, bud outgrowth is strongly governed by apical control, and removal of the shoot apex or floral transition releases lateral buds from inhibition. The same mechanism is supported by decapitation studies showing that intact plants maintain repressed lateral buds because the apex sustains height growth and suppresses bud activity through weak sugar absorption and limited auxin export from buds. After decapitation, those buds break dormancy by exporting more auxin and importing more sugar, which explains why topping rapidly initiates compensatory branching rather than merely stopping stem elongation (Sun et al., 2021).
This compensatory response is regulated by a coordinated hormone–sugar network rather than by auxin alone. In chrysanthemum, release from apical dominance coincides with decreased auxin and increased cytokinin in subapical buds, together with reduced expression of branching repressors such as CmBRC1 and CmMAX1. More broadly, rapid cytokinin accumulation after tip removal appears to be associated with enhanced sugars during the early bud-release phase, while gibberellin contributes more strongly to sustained post-release growth (Cao et al., 2023). This staged view helps explain why stronger or repeated topping usually increases branch number: each removal event reopens dormant buds and renews competitive branch establishment across the canopy.
7.2 Canopy restructuring and photosynthetic productivity
Once buds are released, topping reshapes the canopy by reducing vertical dominance and expanding lateral spread, which changes light interception and the distribution of assimilatory surface. Field studies in chrysanthemum show that no pinching generally maintains the greatest plant height, whereas pinching at 30-40 days after transplanting increases branch number, stem girth, or plant spread depending on treatment timing. Repeated pinching intensifies this structural shift, producing shorter but wider and more highly branched canopies than the control (Ehsanullah et al., 2021). Because canopy architecture governs internal light distribution and resource-use efficiency, these morphological changes are not only geometric but functional for biomass production and flower formation.
The physiological benefit of canopy restructuring depends on whether added branches improve productive light capture more than they increase self-shading. Moderate canopy closure in edible chrysanthemum improved photosynthesis-related traits and increased flower yield, showing that a partially moderated light environment can enhance rather than reduce productivity. In Hangbaiju, branch-promoting regulation by 6-BA plus Pro-Ca increased leaf chlorophyll content and raised flower yield, indicating that architectural control and leaf physiological status can improve together during the floral growth phase. Topping therefore raises yield most effectively when it creates a canopy with enough lateral leaf area and branch spread to intercept light efficiently without imposing excessive mutual shading or an overly long vegetative delay.
7.3 Coupling mechanisms of branch formation, flower bud differentiation, and yield formation
The yield effect of topping ultimately depends on how newly formed branches are converted into reproductive shoots. In Hangbaiju, flower yield depends strongly on shoot branch number because flowers are borne terminally, so each additional successful branch can become an added inflorescence-bearing unit. Across chrysanthemum genotypes, branching and flowering traits vary together, and highly branching material can also show high flower number per plant, confirming that reproductive output is closely tied to shoot architecture rather than to stem elongation alone (Bala and Kaur, 2026). At the developmental level, axillary meristem formation is itself a decisive step in branching capacity, and KNOX genes appear to promote bud formation partly by enhancing the cytokinin pathway while suppressing auxin and gibberellin pathways.
The key trade-off is that topping usually increases the number of reproductive sites while delaying floral transition and redistributing assimilates among more sinks. Double or repeated pinching often increases flowers per plant and total yield, but unpinched plants typically initiate flower buds earlier and flower sooner. This developmental coupling is consistent with chrysanthemum flowering regulators: CmTFL1c delays flowering, promotes axillary bud formation, and alters inflorescence architecture, showing that branching and reproductive timing are mechanistically linked rather than independent traits. Under controlled photoperiods, the same balance reappears agronomically, with no pinch favoring earlier bud initiation and double pinch favoring more branches and flowers, so the best topping method is the one that optimizes branch-derived flowering sites without delaying harvest beyond the production goal. Taken together, different topping methods affect flower yield through an integrated sequence of bud release, canopy reconstruction, and reproductive conversion of lateral shoots. For Hangbaiju, the most productive treatment is therefore not simply the one with the strongest branching response, but the one that best coordinates branching compensation with efficient canopy function and timely flower-bud formation.
8 Production Applications and Optimized Cultivation Strategies
8.1 Selection of topping methods for different production objectives
For production systems targeting early flowering and larger individual flowers, lighter topping or no topping is generally more suitable than repeated pinching. In annual chrysanthemum, no pinching gave the earliest flower bud appearance and the largest flower diameter, even though branch number and total flower number were lower than under stronger pinching treatments. A similar trade-off was reported in Dendranthema grandiflorum cv. Pusa Shwet, where no pinching produced the longest plants, the longest internodes, and the earliest bud appearance, while double pinching increased flowers per stem (Kaur and Singh, 2024). For balanced commercial performance, single pinching often remains a practical compromise, because single pinching at 30 days after transplanting gave satisfactory flower characters in one study, whereas single pinching at 40 days improved shelf life in spray chrysanthemum.
When the objective is to maximize branch number, flower number, and loose-flower yield, repeated pinching is usually superior. Double pinching increased flower number and yield in several annual chrysanthemum studies, and was explicitly recommended for commercial cultivation where total production is the main target. In spray chrysanthemum, however, the agronomic optimum was not always the most severe treatment: thrice pinching produced the strongest vegetative branching response, but pinching twice at 30 and 40 days gave the highest flower number and yield by weight. For Chrysanthemum morifolium cv. Ratlam Selection, pinching at 30 days after transplanting also improved branch number and plant spread, supporting the use of an earlier, moderate topping regime when canopy expansion is prioritized without excessive flowering delay.
8.2 Synergistic regulation of topping, planting density, and water and fertilizer management
Pinching responses are strongly shaped by planting density, so topping should be selected together with spacing rather than as an isolated treatment. In annual chrysanthemum, wider spacing increased stem girth and branching, whereas the highest flower yield per hectare was obtained at 45 × 30 cm combined with pinching at 30 days after transplanting. In C. morifolium cv. Ratlam Selection, wider spacing plus pinching at 30 days increased branches and plant spread, while closer spacing accelerated bud initiation and 50% flowering, indicating that density modifies whether the crop favors vegetative expansion or earlier reproductive progression. Planting date also changes the economic optimum, because the highest B:C ratio in one staggered-planting study was obtained with first-week-of-October planting and pinching at 30 days, even though the highest branch number occurred under double pinching.
Fertilizer and growth-regulator management further determine how effectively topped plants convert extra branches into yield. Standard field protocols in chrysanthemum commonly split nitrogen, applying part basally and the remainder around 30 days after transplanting, which aligns nutrient availability with the active regrowth phase after pinching. Nitrogen-response data show that pinching at 20 days combined with 150 kg·N·ha⁻¹ maximized stem diameter, branching, leaf area, and flower yield, indicating that topped plants benefit from stronger nutrient support once apical dominance is removed (Thakare et al., 2020). Comparable synergy appears with growth regulators: double pinching with triacontanol improved vegetative and floral parameters in cv. Pusa Kesari, while GA₃ at 300 ppm combined with pinching at 40 days improved leaves, flowers, and yield per hectare in Punjab conditions.
8.3 Simplified and precision pruning technologies for Hangbaiju
For Hangbaiju, the main production challenge is that branch promotion has traditionally depended on repeated manual decapitation, which is labor-intensive, costly, and associated with higher disease risk. This makes simplified pruning a practical necessity rather than only a refinement of crop management. Because Hangbaiju flowers are borne at branch termini, any simplified pruning method must still preserve high branch numbers if yield is to be maintained. A useful production direction is therefore to replace some manual topping operations with growth-regulating strategies that mimic the branching effect of repeated decapitation while reducing labor inputs.
Current evidence suggests that precision branch regulation in Hangbaiju can be achieved by combining fewer physical interventions with targeted chemical control. In pot-grown Hangbaiju, foliar application of 6-BA combined with Pro-Ca increased flower yield, and the highest yield was recorded in the 6-BA5 + Ca100 treatment in both experimental years. This approach is attractive for precision cultivation because the untreated control still relied on three manual decapitations, whereas the regulator-based system was explicitly tested as an alternative branch-management technology. Beyond yield, Hangbaiju stems are themselves a usable by-product rich in phenolic compounds, so pruning systems that standardize shoot removal could also improve residue collection and downstream valorization (Zhu et al., 2024). Overall, optimized Hangbaiju production depends on choosing the topping method that matches the production objective, then integrating it with spacing, nutrient scheduling, and labor-saving branch regulation. For most commercial loose-flower systems, moderate or repeated topping appears most effective for maximizing productive branching, but simplified precision approaches are likely to be the most sustainable long-term strategy for Hangbaiju.
9 Conclusions and Perspectives
Different topping methods consistently reshaped Hangbaiju architecture by weakening apical dominance and promoting axillary bud outgrowth. Single topping usually produced a moderate increase in branch number and canopy spread, while repeated topping generated more primary and secondary branches and a denser shoot system. The overall pattern shows that topping intensity controls how strongly vegetative growth is redirected from the main stem to lateral shoots. The branching response also depended on topping timing. Early topping tended to trigger earlier and stronger lateral bud release, whereas later or repeated topping often produced a more compact but more highly branched plant type. These differences indicate that branch formation is not determined by topping alone, but by the interaction between pruning intensity, developmental stage, and cultivar response.
Topping influenced flower yield mainly by changing the number of flowering branches and the balance between vegetative growth and reproductive development. Moderate topping often improved total flower number and yield because it increased the number of terminal flowering sites without excessively delaying flowering. In contrast, no topping favored earlier bud initiation and larger individual flowers, but generally produced fewer flowers per plant. Repeated topping usually increased total yield more strongly than single topping when the production goal was loose-flower output. However, too many topping events could prolong the vegetative phase and redistribute assimilates across too many shoots, which may reduce uniformity or delay harvest. The best treatment therefore depends on whether the target is early flowering, large flowers, or maximum total flower yield.
Current evidence still has several limitations. Most studies focus on a limited number of topping schedules, cultivars, and environments, so results cannot be generalized to all Hangbaiju production systems. Many reports also emphasize morphology and yield, while fewer examine hormone regulation, carbon allocation, canopy photosynthesis, and long-term field performance in an integrated way. Future research should combine topping with plant density, fertilization, irrigation, and growth-regulator management to define optimal production packages. More work is also needed on simplified and precision pruning methods that reduce labor while preserving yield. At the mechanistic level, studies integrating transcriptomics, hormone profiling, and canopy physiology would clarify how topping regulates branch development and floral formation.
Acknowledgments
I extend my sincere gratitude to the anonymous reviewers for their valuable and insightful comments, which have greatly strengthened this paper.
Conflict of Interest Disclosure
The author affirms that this research was conducted without any commercial or financial relationships that could be construed as a potential conflict of interest.
Bala M., and Kaur K., 2026, Morphological and reproductive trait analysis for assessment of genetic diversity in Chrysanthemum morifolium Ramat., BMC Plant Biology, 26(1): 1225.
https://doi.org/10.1186/s12870-026-08824-z
Cao D., Chabikwa T., Barbier F., Dun E.A., Fichtner F., Dong L., Kerr S.C., and Beveridge C.A., 2023, Auxin-independent effects of apical dominance induce changes in phytohormones correlated with bud outgrowth, Plant Physiology, 192(2): 1420-1434.
https://doi.org/10.1093/plphys/kiad034
Chandio S.R., Meghwar M.R., Shar A.B., Wagan M.A., and Shar I.A., 2023, Effect of pinching on growth and yield of marigold, Big Data in Agriculture, 5(2): 53-56.
https://doi.org/10.26480/bda.02.2023.53.56
Das R., and Patra S.K., 2025, Influence of pinching on growth and flowering of spray type of chrysanthemum (Dendranthema grandiflora) cv. Shyamal, Ecology, Environment and Conservation, 31(4): 1404.
https://doi.org/10.53550/EEC.2025.v31i04.011
Ehsanullah M., Tarapder S.A., Maukeeb A.R.M., Khan A.U., and Khan A.U., 2021, Effect of pinching on growth and quality flower production of chrysanthemum (Chrysanthemum indicum L.), Journal of Multidisciplinary Applied Natural Science, 1(2): 62-68.
https://doi.org/10.47352/jmans.v1i2.15
Jena S., Mohanty C.R., Patra C., and Dash R.M., 2021, Effect of pinching on growth and flowering of annual chrysanthemum (Chrysanthemum coronarium L.), Journal of Pharmacognosy and Phytochemistry, 10(2): 1042-1045.
Kathad S.V., Masu M.M., Parekh D.D., and Bagadia I.K., 2024, Effect of different plant spacing and time of pinching on growth and flowering of chrysanthemum (Chrysanthemum morifolium L.) cv. Ratlam Selection, International Journal of Advanced Biochemistry Research, 8(7): 1060-1063.
https://doi.org/10.33545/26174693.2024.v8.i7m.1665
Kaur J., and Singh J., 2024, Effect of pinching and growth regulators on vegetative growth, flowering and pot presentability of chrysanthemum (Dendranthema grandiflorum) cv. Pusa Shwet, Ecology, Environment and Conservation, 30(1): 88-91.
https://doi.org/10.53550/eec.2024.v30i01.016
Sahu J.K., Sahu D., Kispotta G.S., and Nag K., 2024, Effects of pinching and plant growth regulators on chrysanthemum productivity in the central plain zone of Punjab, Environment Conservation Journal, 25(2): 575-580.
https://doi.org/10.36953/ECJ.25362712
Liu H., Wu Y., Lu J., Gou T., Zhao S., Chen F., Chen S., Fang W., and Guan Z., 2025, Predictive modeling study on the critical nitrogen concentration and accumulation in cut chrysanthemum based on the cumulative photo-thermal effect, Horticulturae, 11(11): 1313.
https://doi.org/10.3390/horticulturae11111313
Mangulal R., Laxminarayana D., Prasanth P., Jyothi G., and Praneeth Kumar S., 2025, Effect of pinching and plant growth retardants on vegetative growth of annual chrysanthemum (Glebionis coronaria L.) under Central Telangana conditions, Plant Archives, 2025: 2517-2522.
https://doi.org/10.51470/PLANTARCHIVES.2025.v25.no.2.359
Matsunaga A., and Sasaki H., 2026, Lateral shoot development response to multi-pinching in the garland chrysanthemum cultivar ‘Stick-syungiku’, The Horticulture Journal, 95(2): 245-253.
https://doi.org/10.2503/hortj.SZD-075
Mohanty M., Mohanty C.R., Jena S., and Mohanty S., 2025, Impact of pinching on growth and flowering of annual chrysanthemum (Chrysanthemum coronarium L.), Ecology, Environment and Conservation, 31: S141.
https://doi.org/10.53550/eec.2025.v31i01s.026
Nagdeve N.S., Khobragade H.M., Thakare A., Gajbhiye R.P., and Mandhare K.S., 2021, Effect of plant spacing and pinching on growth and flower yield of annual chrysanthemum, International Journal of Chemical Studies, 9(1): 491-495.
https://doi.org/10.22271/chemi.2021.v9.i1g.11279
Nateshkumar A., Indhumathi K., Arunkumar R., Chitra R., Sangeetha M., and Hariraj N., 2025, Impact of canopy architecture on phenology and production efficiency of flower crops: A review, Plant Science Today, 12: 1-11.
https://doi.org/10.14719/pst.10508
Ran H., 2025, 3D model-based simulation of plum tree canopy light interception, Proceedings of the 2025 International Conference on Smart Agriculture and Artificial Intelligence, 2025: 41-46.
https://doi.org/10.1145/3767624.3767631
Sun D., Zhang L., Su J., Yu Q., Zhang J., Fang W., Wang H., Guan Z., Chen F., and Song A., 2022, Genetic diversity and genome-wide association study of architectural traits of spray cut chrysanthemum varieties, Horticulturae, 8(5): 458.
https://doi.org/10.3390/horticulturae8050458
Sun D., Zhang L., Yu Q., Zhang J., Li P.L., Zhang Y., Xing X., Ding L., Fang W., Chen F., and Song A., 2021, Integrated signals of jasmonates, sugars, cytokinins and auxin influence the initial growth of the second buds of chrysanthemum after decapitation, Biology, 10(5): 440.
https://doi.org/10.3390/biology10050440
Thakare A.A., Dahale M.H., Deogade A.S., Ingole A.R., and Ningot E.P., 2020, Effect of pinching and nitrogen on growth and flower yield of annual chrysanthemum, Journal of Pharmacognosy and Phytochemistry, 9(6): 945-949.
Thumar B.V., Chovatiya N.V., Butani A.M., Bhalu V.B., and Jindal M., 2020, Effect of planting time and pinching on flowering and yield of chrysanthemum (Dendranthema grandiflora) cv. Ratlam selection, Journal of Pharmacognosy and Phytochemistry, 9(2): 414-416.
Wang F., Hu Z., Luo H., Wu Q., Chen X., Wen S., Xiao Z., Ai X., and Guo Y., 2024, The functional verification of CmSMXL6 from chrysanthemum in the regulation of branching in Arabidopsis thaliana, Horticulturae, 10(7): 718.
https://doi.org/10.3390/horticulturae10070718
Yang F., Shao W.Q., Lu X.Y., Ying L., and Huang C., 2024, Improving effect of agroforestry intercropping on the quality and yield of edible chrysanthemums, Applied Ecology and Environmental Research, 22(2): 1087.
https://doi.org/10.15666/aeer/2202_10871105
Yuan T.L., Tian T., Chen Z., Ye T., Zhu X.H., Song G.S., Wang D.L., Li L., Cheng Y., and Gong J.Y., 2025, Extraction of polyphenols from Chrysanthemum morifolium Ramat. leaves, Industrial Crops and Products, 231: 121221.
https://doi.org/10.1016/j.indcrop.2025.121221
Zhang Y.Q., Guo C., Hu J., Liu F.Y., Fu S., Guo X.M., Chen Q., Zhang L., Zhu L.X., and Hou X., 2023, Effects of 6-benzylaminopurine combined with prohexadione-Ca on yield and quality of Chrysanthemum morifolium Ramat cv. Hangbaiju, Agriculture, 13(2): 444.
https://doi.org/10.3390/agriculture13020444
Zhu X.H., Yuan T.L., Li X., Wang Y.J., Wang D.L., Song G.S., Li L., and Gong J.Y., 2024, Valorization of Chrysanthemum morifolium Ramat. cv. “Hangbaiju” stems for phenolic compounds production by steam explosion pretreatment, Industrial Crops and Products, 213: 118410.
https://doi.org/10.1016/j.indcrop.2024.118410
. PDF(851KB)
. FPDF(win)
. FPDF(mac)
. HTML
. Online fPDF
Associated material
. Readers' comments
Other articles by authors
. Chengbin Jiang

Related articles
. Hangbaiju
. Topping methods
. Branch formation
. Flower yield
. Plant architecture
Tools
. Email to a friend
. Post a comment